Brief Report
Association Between HERC2 rs12913832 Genotype and Eye-colour Phenotype in an Iraqi Sample: A Secondary Data Analysis 
 ,
Kushal Budha
 Author Correspondence author
Biological Evidence, 2026, Vol. 16, No. 5 doi: 10.5376/be.2026.16.0026
Received: 26 Aug., 2026 Accepted: 14 Sep., 2026 Published: 19 Sep., 2026
Lagun N., and Budha K., 2026, Association between HERC2 rs12913832 genotype and eye-colour phenotype in an Iraqi sample: a secondary data analysis, Bioscience Evidence, 16(5): 345-352 (doi: 10.5376/be.2026.16.0026)
Human eye colour is a complex pigmentation phenotype in which HERC2 rs12913832 has one of the strongest known single-variant associations, yet a large genetic effect does not imply one-to-one assignment of categorical eye colour. The original Iraqi IrisPlex pilot study evaluated the combined six-SNP prediction system; here, we performed a focused secondary analysis that isolates rs12913832 and directly quantifies its association with the recorded phenotype categories. Participant-level genotype and observed eye-colour data from all 58 Iraqi individuals were analysed as G/G, G/A, and A/A versus blue, intermediate, and brown eye colour in a 3×3 contingency framework. Because expected cell counts were sparse, the primary analysis used a two-sided Fisher–Freeman–Halton exact test, with Cramér's V as the effect-size measure and Pearson's chi-square as a sensitivity analysis. Eye colour comprised 7 blue, 25 intermediate, and 26 brown phenotypes; genotype counts were 18 G/G, 19 G/A, and 21 A/A. Genotype and phenotype were substantially associated (exact p=4.99×10⁻¹⁰; Cramér's V=0.60), with concordant Pearson evidence (χ²(4, N=58) =42.28, p=1.46×10⁻⁸). All blue-eyed participants were G/G, and 19 of 21 A/A participants were brown-eyed, while the heterogeneous intermediate category occurred in every genotype class. These findings provide a transparent population-specific estimate of the rs12913832-eye-colour association in this Iraqi pilot dataset while showing that the recorded three-category phenotype is not uniquely determined by genotype at this single locus.
1 Introduction
Human iris colour arises from variation in the amount, distribution, and optical effects of melanin within the iris. Although blue and brown eyes are often used as simple examples of inheritance, genetic and quantitative-phenotyping studies show that eye colour is a complex, highly heritable phenotype influenced by multiple loci, with broad colour categories capturing only part of the underlying biological variation (Sturm and Larsson, 2009; Liu et al., 2010; Simcoe et al., 2021). This distinction is important because dominance describes the relationship between alleles at a defined locus, whereas the visible frequency or appearance of a complex phenotype does not by itself establish a one-gene dominant/recessive mechanism.
Among the loci contributing to normal eye-colour variation, the HERC2-OCA2 region on chromosome 15 has one of the largest and most reproducible effects. Association and haplotype studies have established a major contribution of this region to blue-brown eye-colour variation (Duffy et al., 2007; Sturm et al., 2008). The rs12913832 variant, located within an intronic regulatory region of HERC2, has functional evidence linking allelic state to long-range enhancer-promoter interactions and transcriptional regulation of the neighbouring OCA2 gene (Visser et al., 2012). Population-genetic analyses further demonstrate geographic and allelic heterogeneity across the OCA2-HERC2 region, cautioning against assuming that a particular allele label carries identical phenotypic implications across populations (Donnelly et al., 2012).
The same biological architecture underpins forensic DNA phenotyping. IrisPlex incorporates rs12913832 with five additional pigmentation-associated markers to estimate probabilities of blue, intermediate, and brown eye colour (Walsh et al., 2011), and subsequent validation demonstrated strong predictive performance for blue and brown categories across European populations (Walsh et al., 2012). Quantitative analyses nevertheless show considerable within-category and within-genotype variation (Andersen et al., 2013), while analyses of phenotypically discordant rs12913832 genotypes have identified additional variation within the OCA2-HERC2 region that may contribute to eye-colour differences (Salvo et al., 2023). Prediction performance may also vary with population composition, as demonstrated in admixed Latin American populations (Palmal et al., 2021). Together, these findings distinguish a strong locus-level association from the unique assignment of a categorical phenotype.
Al-Rashedi et al. (2020) reported six IrisPlex genotypes, prediction probabilities, and observed eye-colour categories for 58 Iraqi volunteers in a limited pilot study. Their primary objective was to evaluate the performance of the multi-SNP IrisPlex prediction system. The participant-level supplementary data, however, permit a narrower question that was not the primary focus of the original study: how strongly does HERC2 rs12913832 alone correspond to the recorded three-category eye-colour phenotype in this sample? Examining rs12913832 separately allows the observed genotype-phenotype structure to be quantified without conflating it with the multivariable prediction probabilities produced by IrisPlex. The contribution of the present study is therefore not the discovery of a new pigmentation locus but a transparent, population-specific secondary estimate of the strength and pattern of this established association in the available Iraqi pilot dataset, including the extent of within-genotype overlap in the heterogeneous intermediate category. We reanalysed the complete 58-person dataset using one prespecified genetic variant, one observed phenotype, and one primary exact association test. The analytical workflow and provenance are summarised in Figure 1.
|
Figure 1 Analytical workflow and provenance. Participant-level rs12913832 genotype calls and observed eye-colour classifications were extracted from the published Iraqi IrisPlex supplements, verified by Sample ID, and reduced to the prespecified 58-record analysis set. The study was restricted to a 3 × 3 genotype-phenotype table; the Fisher-Freeman-Halton exact test was primary, Cramér's V quantified association magnitude, and Pearson's chi-square was a sensitivity analysis |

2 Results
2.1 Analytical sample and marginal distributions
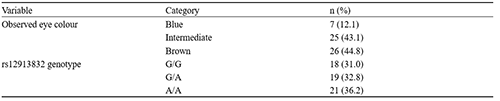
The analytical dataset contained 58 participants with complete rs12913832 genotype and observed eye-colour data; no records were excluded. Blue eye colour was recorded in 7 participants (12.1%), intermediate eye colour in 25 (43.1%), and brown eye colour in 26 (44.8%). Genotype frequencies were G/G in 18 participants (31.0%), G/A in 19 (32.8%), and A/A in 21 (36.2%) (Table 1).
|
Table 1 Distribution of observed eye-colour phenotype and HERC2 rs12913832 genotype Note Percentages use N = 58 as the denominator. No analytical values were missing. |
2.2 Genotype-phenotype distribution
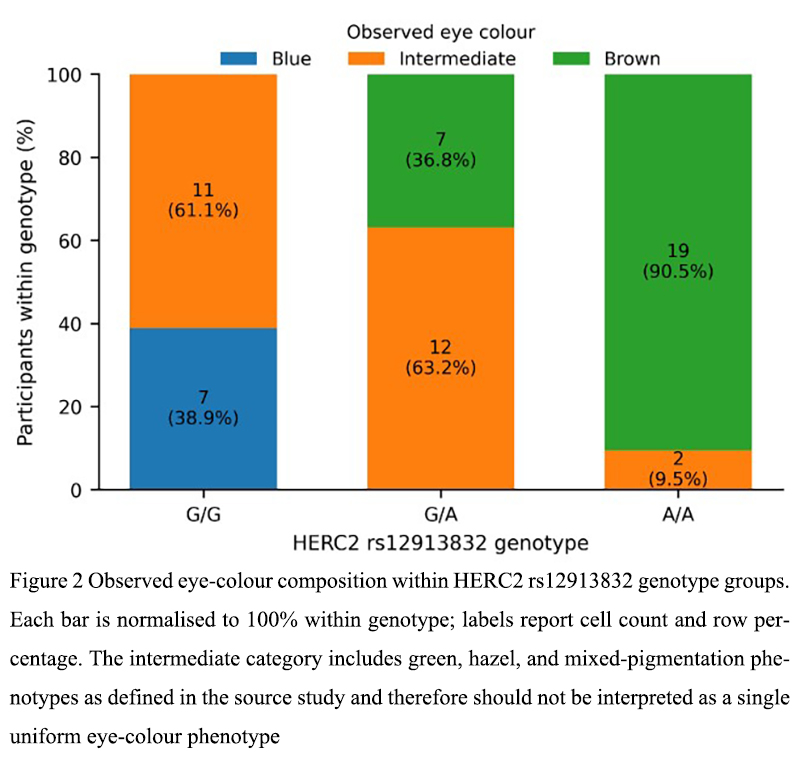
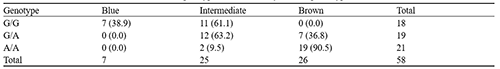
Eye-colour composition differed markedly across genotype groups (Figure 2; Table 2). Among G/G participants, 7 of 18 (38.9%) were blue-eyed and 11 of 18 (61.1%) were intermediate; none was brown-eyed. The G/A group contained 12 of 19 intermediate phenotypes (63.2%) and 7 of 19 brown phenotypes (36.8%), with no blue phenotypes. Among A/A participants, 19 of 21 (90.5%) were brown-eyed and 2 of 21 (9.5%) were intermediate. Viewed from the phenotype side, all seven blue-eyed participants were G/G, whereas 19 of 26 brown-eyed participants (73.1%) were A/A. The intermediate category occurred in all three genotype classes.
|
Figure 2 Observed eye-colour composition within HERC2 rs12913832 genotype groups. Each bar is normalised to 100% within genotype; labels report cell count and row percentage. The intermediate category includes green, hazel, and mixed-pigmentation phenotypes as defined in the source study and therefore should not be interpreted as a single uniform eye-colour phenotype |
|
Table 2 Cross-tabulation of HERC2 rs12913832 genotype and observed eye-colour phenotype Note Values are n (row %) for genotype rows. Fisher–Freeman–Halton exact p = 4.99 × 10⁻¹⁰; Cramér's V = 0.60. |
2.3 Association analysis
Expected cell frequencies under genotype–phenotype independence ranged from 2.17 to 9.41. Three of nine cells (33.3%) had expected counts below 5, including all three expected blue-phenotype cells; this sparse structure supported use of an exact rather than asymptotic test as the primary inferential procedure.
Exhaustive enumeration identified 8,454 feasible 3 × 3 contingency tables with the observed row and column margins. Using a two-sided Fisher-Freeman-Halton exact test with probability ordering (Freeman and Halton, 1951), the observed table had a conditional probability of 4.52×10⁻¹² and the exact association p value was 4.99×10⁻¹⁰. Association magnitude was substantial, with Cramér's V=0.60 (Cramér, 1999). Pearson's chi-square sensitivity analysis produced the same substantive conclusion, χ²(4, N=58)=42.28, p=1.46×10⁻⁸. Thus, the evidence for association did not depend on the asymptotic chi-square approximation.
3 Discussion
3.1 Principal finding and contribution
This focused secondary analysis shows a substantial association between the HERC2 rs12913832 genotype and the recorded eye-colour category in the 58-person Iraqi dataset. The contribution is deliberately narrow: unlike the original study, which evaluated the combined six-SNP IrisPlex prediction system, the present analysis isolates a single established major locus and quantifies its direct contingency structure, effect size, and phenotype overlap in the available Iraqi sample. G/G was confined to blue and intermediate phenotypes, A/A was overwhelmingly concentrated in brown phenotypes, and G/A occupied intermediate and brown categories. At the same time, genotype classes did not map one-to-one onto the three recorded phenotype categories. The result therefore supports a major genotype-phenotype relationship without implying that rs12913832 uniquely determines categorical eye colour.
3.2 Biological interpretation and the intermediate category
The direction of the observed association is consistent with the established importance of the HERC2-OCA2 region in human iris pigmentation. Functional studies have shown that rs12913832 can influence long-range enhancer-promoter interactions and transcriptional regulation of the neighbouring OCA2 gene (Visser et al., 2012), while association and population-genetic studies have identified this region as a major contributor to normal eye-colour variation (Duffy et al., 2007; Sturm et al., 2008; Donnelly et al., 2012). The present analysis does not independently establish this molecular mechanism; it addresses the narrower question of how the established locus corresponds to the recorded phenotype categories in this Iraqi pilot dataset.
The intermediate category requires particular caution. In the source study it included green, hazel, and irises containing combinations of two or more pigments, making it a phenotypically heterogeneous operational category rather than a single uniform eye-colour phenotype (Al-Rashedi et al., 2020). Broad categorical labels also compress continuous variation in iris pigmentation (Liu et al., 2010; Andersen et al., 2013). Accordingly, the presence of intermediate phenotypes in all three genotype classes should not be interpreted as direct evidence that any specific additional locus explains an individual discordant case. The overlap is consistent with the established polygenic architecture of pigmentation, but it may also reflect information loss from coarse phenotypic categorisation and other unmeasured sources of variation. Additional OCA2-HERC2 variation and interactions among pigmentation-associated genes remain biologically plausible contributors (Branicki et al., 2009; Salvo et al., 2023).
3.3 Population context, strengths, and limitations
The extent to which the observed genotype-phenotype pattern applies beyond this dataset cannot be determined from a 58-person pilot sample. Pigmentation architecture can vary with ancestry and population history, and studies in admixed populations have identified multiple independent signals within and beyond the OCA2-HERC2 region (Adhikari et al., 2019). Broader reviews likewise emphasise allelic and locus heterogeneity across populations (Liu et al., 2013), while epistatic interactions can influence DNA-based pigmentation prediction (Pośpiech et al., 2014). The original Iraqi study itself was presented as a limited pilot investigation and recommended larger samples before population-level conclusions were drawn (Al-Rashedi et al., 2020). The present result should therefore be interpreted as a dataset-level association, not as an estimate of rs12913832 penetrance or eye-colour distribution for the Iraqi population as a whole.
Strengths of the present analysis include its prespecified narrow scope, complete participant-level genotype and phenotype data, exact inference matched to the sparse 3 × 3 table, and a locked reproducibility workflow linking the published source supplement to the derived analysis. Limitations are inherited largely from the source study: the sample is small; recruitment, phenotype assessment, and laboratory procedures could not be controlled by the present investigators; eye colour was recorded in three broad categories rather than quantitatively; the published eye photographs were not independently reclassified; ancestry covariates suitable for population-structure adjustment were unavailable; and the single-SNP design cannot identify which additional loci or interactions contribute to intermediate or otherwise discordant phenotypes. Statistical precision and generalisability are therefore limited, and the observed association should not be interpreted as evidence that rs12913832 causally determines an individual's eye colour.
3.4 Implications
The findings do not challenge the established importance of rs12913832. Instead, they provide a reproducible population-specific illustration of how a large-effect pigmentation-associated variant can show a strong association while retaining within-genotype categorical overlap. Larger studies involving Iraqi and neighbouring populations could test whether the same distribution persists in more representative samples and after adjustment for ancestry. Future work could also combine rs12913832 with additional pigmentation-associated loci and quantitative iris imaging to characterise variation obscured by broad categorical phenotypes. Such studies would extend the present result without conflating high associative or predictive informativeness at a major locus with a simple one-locus genotype-to-phenotype rule.
4 Methods
4.1 Study design and data source
We conducted a secondary analysis of participant-level data from the Iraqi IrisPlex pilot study reported by Al-Rashedi et al. (2020). The original study enrolled 58 Iraqi volunteers, genotyped six established IrisPlex markers using the Sequenom MassARRAY platform, and reported participant-level genotypes, eye-colour prediction probabilities, and observed eye-colour classifications in the accompanying supplementary materials. The present analysis was deliberately restricted to the HERC2 rs12913832 genotype and the corresponding observed eye-colour phenotype. No new participants were recruited, no biological specimens were collected, and no additional genotyping or phenotyping was performed.
4.2 Ethical context
The original investigators reported ethical approval from the Ethics Committee of Al-Muthanna University (Document No. 2032, dated 10 May 2018) and written informed consent from all participants (Al-Rashedi et al., 2020). The present study used only participant-level data already available in the published article and its supplementary materials. No direct participant contact, additional biological sampling, or new data collection occurred. Accordingly, this study does not claim new ethical approval or exemption for the secondary analysis.
4.3 Eye-colour phenotype
The original study classified observed eye colour into blue, intermediate, and brown categories. Shades of blue were grouped as blue and shades of brown as brown; green, hazel, and irises containing combinations of two or more pigments were classified as intermediate (Al-Rashedi et al., 2020). Thus, the intermediate category was intrinsically heterogeneous. Eye photographs were collected by the original investigators as supporting documentation. The present analysis used the recorded phenotype classifications from the source dataset and did not independently reclassify the photographs, avoiding the introduction of an additional subjective phenotype-assessment layer.
4.4 rs12913832 genotype and strand convention
Participant-level rs12913832 genotype calls were obtained from the published supplementary data. Supplementary Table 2 reported the calls as G, GA, and A, which were standardised in the analytical dataset as G/G, G/A, and A/A, respectively. The supplementary data also included an rs12913832_T numerical field used in the IrisPlex representation. Cross-checking all 58 participant records confirmed internally consistent 0/1/2 coding between the genotype and phenotype source tables.
Because rs12913832 may be represented using genomic A/G or reverse-strand C/T nomenclature, the A/G convention used in the source dataset was retained throughout. Allelic direction was not inferred across external studies unless strand orientation was explicitly established, reducing the risk of strand-related misinterpretation.
4.5 Data extraction and analytical sample
Participant identifiers were matched across the genotype and phenotype supplementary tables. For each individual, the standardised rs12913832 genotype and corresponding observed eye-colour category were extracted. All 58 participant identifiers were unique, complete genotype and phenotype information was available for every individual, and no records were excluded. Before statistical testing, genotype and phenotype totals were independently checked against the source supplementary data to confirm consistency with the published records.
4.6 Statistical analysis
Descriptive statistics were calculated for the three eye-colour categories and three rs12913832 genotype groups and are reported as counts and percentages. Genotype and phenotype were cross-tabulated in a 3 × 3 contingency table, and expected cell frequencies under the null hypothesis of independence were calculated from the observed marginal totals.
Because three of nine expected cell frequencies were below 5, the primary inferential procedure was the Fisher-Freeman-Halton exact test, the extension of Fisher's exact test to r×c contingency tables (Freeman and Halton, 1951). A two-sided exact p value was obtained by exhaustive enumeration of all feasible contingency tables with the observed row and column margins. Using probability ordering, probabilities of all tables with conditional probability less than or equal to that of the observed table were summed to obtain the exact two-sided significance level. Statistical significance was prespecified at α=0.05, two-sided. Association magnitude was quantified using Cramér's V (Cramér, 1999). Pearson's chi-square test was retained as a sensitivity analysis rather than a co-primary test because of the sparse expected-cell structure. No multiple-testing correction was applied because only one primary hypothesis test was prespecified.
4.7 Reproducibility
The analytical CSV, extraction script, and analysis script constitute the authoritative computational record for the present study. The workflow reads the locked 58-participant dataset and regenerates the descriptive distributions, 3 × 3 contingency table, expected cell counts, Fisher-Freeman-Halton exact test, Pearson chi-square sensitivity analysis, Cramér's V, and the genotype-specific stacked phenotype figure from the same source data. Analyses involving the other five IrisPlex SNPs, sex-stratified modelling, regression, ROC/AUC analysis, machine-learning approaches, epistasis testing, image-based phenotype reclassification, and ancestry modelling were outside the prespecified scope and were not performed.
5 Conclusion
In this secondary analysis of 58 Iraqi participants, the HERC2 rs12913832 genotype was substantially associated with recorded blue, intermediate, and brown eye-colour categories (exact p=4.99×10⁻¹⁰; Cramér's V=0.60). The association was marked, but phenotype overlap remained within genotype classes, particularly within the heterogeneous intermediate category. The result is consistent with rs12913832 being a major eye-colour-associated locus while showing that the recorded three-category phenotype is not uniquely determined by genotype at this single locus. Because the source dataset was a small pilot sample, these findings should be treated as a reproducible dataset-level secondary estimate rather than a population-wide or causal inference for Iraq.
Declarations
Data availability
The participant-level source data used in this secondary analysis are available in the published article and supplementary materials of Al-Rashedi et al. (2020). The derived 58-participant analytical dataset used for the present study is included in the accompanying reproducibility package.
Code availability
The reproducibility package contains the extraction script, locked analytical CSV, analysis script, results summary, tables, figure, and analysis notes required to regenerate the reported core results. The package is available from Zenodo: https://doi.org/10.5281/zenodo.22106141.
Ethics statement
No new participants were recruited, no new biological specimens were collected, and no additional participant contact occurred in the present secondary analysis. The original investigators reported approval from the Ethics Committee of Al-Muthanna University (Document No. 2032, dated 10 May 2018) and stated that written informed consent was obtained from all participants (Al-Rashedi et al., 2020). The present study was restricted to secondary analysis of participant-level data already available in the published article and supplementary materials.
Author contributions
N.L. conceived and designed the study, developed the methodology, curated and analysed the data, conducted the formal statistical analysis, prepared the visualisations, interpreted the findings, and drafted the manuscript. K.B. contributed to the investigation, interpretation of the findings, and critical revision of the manuscript for important intellectual content. Both authors reviewed and approved the final version and accept responsibility for the work.
Adhikari K., Mendoza-Revilla J., Sohail A., Fuentes-Guajardo M., Lampert J., Chacón-Duque J. C., Hurtado M., Villegas V., Granja V., Acuña-Alonzo V., Jaramillo C., Arias W., Barquera Lozano R., Everardo P., Gómez-Valdés J., Villamil-Ramírez H., Silva de Cerqueira C. C., Hunemeier T., Ramallo V., Schuler-Faccini L., Salzano F. M., Gonzalez-José R., Bortolini M. C., Canizales-Quinteros S., Gallo C., Poletti G., Bedoya G., Rothhammer F., Tobin D. J., Fumagalli M., Balding D., and Ruiz-Linares A., 2019, A GWAS in Latin Americans highlights the convergent evolution of lighter skin pigmentation in Eurasia, Nature Communications, 10(1): 358.
https://doi.org/10.1038/s41467-018-08147-0
Al-Rashedi N. A., Mandal A. M., and ALObaidi L. A., 2020, Eye color prediction using the IrisPlex system: a limited pilot study in the Iraqi population, Egyptian Journal of Forensic Sciences, 10(1): 27.
https://doi.org/10.1186/s41935-020-00200-8
Andersen J. D., Johansen P., Harder S., Christoffersen S. R., Delgado M. C., Henriksen S. T., Nielsen M. M., Sørensen E., Ullum H., Hansen T., Dahl A. L., Paulsen R. R., Børsting C., and Morling N., 2013, Genetic analyses of the human eye colours using a novel objective method for eye colour classification, Forensic Science International: Genetics, 7(5): 508-515.
https://doi.org/10.1016/j.fsigen.2013.05.003
Branicki W., Brudnik U., and Wojas-Pelc A., 2009, Interactions between HERC2, OCA2 and MC1R may influence human pigmentation phenotype, Annals of Human Genetics, 73(2): 160-170.
https://doi.org/10.1111/j.1469-1809.2009.00504.x
Cramér H., 1999, Mathematical Methods of Statistics, Princeton University Press, Princeton, USA.
https://doi.org/10.1515/9781400883868
Donnelly M.P., Paschou P., Grigorenko E., Gurwitz D., Barta C., Lu R.B., Zhukova O.V., Kim J.J., Siniscalco M., New M., Li H., Kajuna S.L.B., Manolopoulos V.G., Speed W.C., Pakstis A. J., Kidd J.R., and Kidd K.K., 2012, A global view of the OCA2-HERC2 region and pigmentation, Human Genetics, 131(5): 683-696.
https://doi.org/10.1007/s00439-011-1110-x
Duffy D.L., Montgomery G.W., Chen W., Zhao Z.Z., Le L., James M.R., Hayward N.K., Martin N.G., and Sturm R.A., 2007, A three-single-nucleotide polymorphism haplotype in intron 1 of OCA2 explains most human eye-color variation, The American Journal of Human Genetics, 80(2): 241-252.
https://doi.org/10.1086/510885
Freeman G.H., and Halton J.H., 1951, Note on an exact treatment of contingency, goodness of fit and other problems of significance, Biometrika, 38(1/2): 141-149.
https://doi.org/10.1093/biomet/38.1-2.141
Liu F., Wen B., and Kayser M., 2013, Colorful DNA polymorphisms in humans, Seminars in Cell & Developmental Biology, 24(6-7): 562-575.
https://doi.org/10.1016/j.semcdb.2013.03.013
Liu F., Wollstein A., Hysi P.G., Ankra-Badu G.A., Spector T.D., Park D., Zhu G., Larsson M., Duffy D.L., Montgomery G.W., Mackey D.A., Walsh S., Lao O., Hofman A., Rivadeneira F., Vingerling J.R., Uitterlinden A.G., Martin N.G., Hammond C.J., and Kayser M., 2010, Digital quantification of human eye color highlights genetic association of three new loci, PLoS Genetics, 6(5): e1000934.
https://doi.org/10.1371/journal.pgen.1000934
Palmal S., Adhikari K., Mendoza-Revilla J., Fuentes-Guajardo M., de Cerqueira C.C.S., Bonfante B., Chacón-Duque J.C., Sohail A., Hurtado M., Villegas V., Granja V., Jaramillo C., Arias W., Barquera Lozano R., Everardo-Martínez P., Gómez-Valdés J., Villamil-Ramírez H., Hünemeier T., Ramallo V., Parolin M.L., and Ruiz-Linares A., 2021, Prediction of eye, hair and skin colour in Latin Americans, Forensic Science International: Genetics, 53: 102517.
https://doi.org/10.1016/j.fsigen.2021.102517
Pośpiech E., Wojas-Pelc A., Walsh S., Liu F., Maeda H., Ishikawa T., Skowron M., Kayser M., and Branicki W., 2014, The common occurrence of epistasis in the determination of human pigmentation and its impact on DNA-based pigmentation phenotype prediction, Forensic Science International: Genetics, 11: 64-72.
https://doi.org/10.1016/j.fsigen.2014.01.012
Salvo N. M., Andersen J. D., Janssen K., Meyer O. L., Berg T., Børsting C., and Olsen G. H., 2023, Association between variants in the OCA2-HERC2 region and blue eye colour in HERC2 rs12913832 AA and AG individuals, Genes, 14(3): 698.
https://doi.org/10.3390/genes14030698
Simcoe M., Valdes A., Liu F., Furlotte N.A., Evans D.M., Hemani G., Ring S.M., Smith G.D., Duffy D.L., Zhu G., Gordon S.D., Medland S. E., Vuckovic D., Girotto G., Sala C., Catamo E., Concas M. P., Brumat M., Gasparini P., Toniolo D., Cocca M., Robino A., Yazar S., Hewitt A., Wu W., Kraft P., Hammond C. J., Shi Y., Chen Y., Zeng C., Klaver C. C. W., Uitterlinden A.G., Ikram M. A., Hamer M. A., van Duijn C. M., Nijsten T., Han J., Mackey D. A., Martin N. G., Cheng C. Y., the 23andMe Research Team, the International Visible Trait Genetics Consortium, Hinds D. A., Spector T.D., Kayser M., and Hysi P. G., 2021, Genome-wide association study in almost 195,000 individuals identifies 50 previously unidentified genetic loci for eye color, Science Advances, 7(11): eabd1239.
https://doi.org/10.1126/sciadv.abd1239
Sturm R. A., and Larsson M., 2009, Genetics of human iris colour and patterns, Pigment Cell & Melanoma Research, 22(5): 544-562.
https://doi.org/10.1111/j.1755-148X.2009.00606.x
Sturm R. A., Duffy D. L., Zhao Z. Z., Leite F. P., Stark M. S., Hayward N. K., Martin N. G., and Montgomery G. W., 2008, A single SNP in an evolutionary conserved region within intron 86 of the HERC2 gene determines human blue-brown eye color, American Journal of Human Genetics, 82(2): 424-431.
https://doi.org/10.1016/j.ajhg.2007.11.005
Visser M., Kayser M., and Palstra R. J., 2012, HERC2 rs12913832 modulates human pigmentation by attenuating chromatin-loop formation between a long-range enhancer and the OCA2 promoter, Genome Research, 22(3): 446-455.
https://doi.org/10.1101/gr.128652.111
Walsh S., Liu F., Ballantyne K. N., Van Oven M., Lao O., and Kayser M., 2011, IrisPlex: a sensitive DNA tool for accurate prediction of blue and brown eye colour in the absence of ancestry information, Forensic Science International: Genetics, 5(3): 170-180.
https://doi.org/10.1016/j.fsigen.2010.02.004
Walsh S., Wollstein A., Liu F., Chakravarthy U., Rahu M., Seland J. H., Soubrane G., Tomazzoli L., Topouzis F., Vingerling J. R., Vioque J., Fletcher A. E., Ballantyne K. N., and Kayser M., 2012, DNA-based eye colour prediction across Europe with the IrisPlex system, Forensic Science International: Genetics, 6(3): 330-340.
https://doi.org/10.1016/j.fsigen.2011.07.009
. PDF(491KB)
. HTML
Associated material
. Readers' comments
Other articles by authors
. Nikesh Lagun

. Kushal Budha
Related articles
. HERC2
. rs12913832
. Eye colour
. Genotype-phenotype association
. Human pigmentation
. IrisPlex
Tools
. Email to a friend
. Post a comment